Biochemistry of Amino Acids - A. Meister 1961
General Biochemistry and Physiology of Amino Acid Metabolism
Oxidative Deamination
D-Amino Acid Oxidase
In mammals, D-amino acid oxidase is found exclusively in The Liver and Kidney Tissues, with its activity in the Kidneys being significantly higher than in the liver. This enzyme has been obtained in a highly purified state, exhibiting a turnover number ranging from 1,000 to 2,000 per minute [121, 122]. The enzyme oxidizes A wide variety of D-Amino Acids and shows no detectable activity toward L-amino acids. In this context, It is worth noting that it is used to detect trace amounts of D-amino acids in the presence of high concentrations of their corresponding L-isomers (p. 95). Certain Species Differences in the substrate Specificity of the enzyme have been noted; for instance, the relative oxidation rates of various D-amino acids by oxidase preparations from pig and ram kidneys differ slightly. These variations are presumably attributable to the distinct Nature of the apoenzymes.
Renal D-amino acid oxidase is inactive against amino acids in which the α-hydrogen atom or both hydrogen atoms of the amino group are substituted. Table 18 presents selected literature data on the enzymatic oxidation of various amino acids.
Class="center">Table 18 Specificity of Certain amino acid Oxidases
|
Amino acid |
Enzyme activity toward the corresponding amino acid * |
||||
|
L-oxidase from N. crassa [124] |
L-oxidase from rattlesnake venom [123] |
Rat kidney L-oxidase [118] |
Sheep kidney D-oxidase [124] |
Octopus liver D-oxidase [125] |
|
|
53 |
0.4 |
_ |
34 |
53 |
|
|
α-Aminoadipic acid |
78 |
7 |
— |
0 |
— |
|
α-Aminobutyric acid |
82 |
20 |
3 |
16 |
(100) |
|
— |
7 |
— |
— |
— |
|
|
Aspartic acid |
6 |
<0.1 |
0 |
0.5 |
25 |
|
Valine |
8 |
4 |
28 |
18 |
34 |
|
47 |
14 |
9 |
3 |
62 |
|
|
Glutamic acid |
12 |
<0.1 |
0 |
0 |
57 |
|
Isoleucine |
42 |
29 |
71 |
12 |
37 |
|
Leucine |
(100) |
92 |
(100) |
7 |
53 |
|
18 |
0.2 |
0 |
0.3 |
— |
|
|
51 |
(100) |
81 |
42 |
70 |
|
|
65 |
од |
0 |
2 |
— |
|
|
0 |
0 |
77 |
78 |
46 |
|
|
10 |
0 |
0 |
22 |
23 |
|
|
31 |
76 |
20 |
(100) |
— |
|
|
3 |
0 |
0 |
1 |
— |
|
|
35 |
82 |
40 |
19 |
16 |
|
|
Phenylalanine |
53 |
76 |
45 |
14 |
— |
|
Cystine |
72 |
26 |
15 |
1 |
— |
* Maximum activity is taken as 100%.
The D-isomers of tyrosine, methionine, and proline are oxidized most rapidly, whereas glutamic and aspartic acids, cystine, lysine, and threonine are oxidized very slowly or not at all. The ω-N-acyl derivatives of lysine and ornithine are oxidized at a noticeable rate [126–128]. D-allo-Threonine is oxidized faster than D-threonine, and D-isoleucine faster than D-allo-isoleucine. The stereoisomers of isoleucine are oxidized to the corresponding optically pure enantiomorphic forms of α-keto-β-methylvaleric acid; this observation Supports the view that no double bond arises between the α- and β-carbon atoms during The amino acid oxidation process [129, 130]. A similar Conclusion follows from the fact that D-amino acid oxidase oxidizes D-α-aminophenylacetic acid, which lacks an α-hydrogen atom. This enzyme also oxidizes the D-isomers of many non-protein amino acids, including the D-forms of ethionine, cyclohexylalanine, β-2-thienylalanine, S-alkyl derivatives of Cysteine, allo-threonine, α-aminocaproic acid (norleucine), p-aminophenylalanine, α-aminovaleric acid (norvaline), and several others [131–133]. D-Amino acid oxidase oxidizes N-monomethyl-D-amino acids; in the presence of catalase, the reaction proceeds According to the following overall equation [114, 134]:
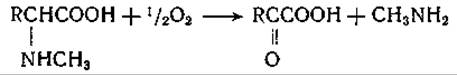
Whether D-amino acid oxidase plays a physiological role and what its exact function might be remains unknown. It is possible that the purpose of this enzyme is to degrade D-amino acids present in the diet or produced within the animal body (for example, As a result of the METABOLIC ACTIVITY OF the bacterial flora in the gastrointestinal tract, Oral Cavity, etc.).
Experiments provide no indication that the synthesis of racemic Amino acids can occur in the animal body; conversely, it has been found that following the ingestion of racemic amino acids labeled with N15, the D-component is excreted in the urine without significant isotope dilution [135]. The activity of D-amino acid oxidase in vivo is supported by several lines of evidence. For instance, it has been established that certain D-amino acids, when administered in the diet instead of the corresponding L-amino acids, support animal growth (p. 135), and that ingestion of certain racemic amino acids results in the urinary excretion of the corresponding α-keto acids [136, 137].
D-Amino acid oxidases have been found in A number of Molds and Bacteria; the substrates for these Enzymes can include D-amino acids occurring in certain microorganisms. Active D-amino acid oxidase preparations have been obtained from Neurospora crassa, Aspergillus niger, Penicillium chrysogenum, Penicillium roqueforti, as well as from various strains of Proteus, Escherichia coli, and Pseudomonas [122, 138–141]. A distinct D-aspartate oxidase has been discovered [142, 143]. This enzyme is found in the liver and kidneys of rabbits and contains flavin adenine dinucleotide (FAD) as a coenzyme. Its action is analogous to that of D-amino acid oxidase. Crude D-amino acid oxidase preparations obtained from pig kidneys may contain D-aspartate oxidase; however, this latter enzyme is inactivated much more readily. D-Aspartate oxidase preparations also oxidize D-glutamic acid, albeit significantly more slowly than aspartic acid. Although the existence of a separate D-glutamate oxidase has been suggested, a clear Separation of D-aspartate and D-glutamate oxidases has not yet been achieved.
D-Glutamate oxidase has been found in the liver of certain cephalopods, including the octopus [125, 144]. This enzyme differs from the oxidase acting on other D-amino acids and also exhibits some activity toward D-aspartic acid.
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.