Chemistry and Biology of Proteins - F. Haurowitz 1953
Protein Complexes with Other Substances
Complexes of Proteins with Non-Protein Components
The Nature of the forces acting in complex Proteins has been studied by combining proteins with various types of substances, particularly anions and cations. The combination of small inorganic ions with proteins was already discussed in Chapter V (see p. 86). It was pointed out there that the ionic groups of proteins combine with calcium cations, phosphate anions, and other inorganic ions through The formation of salt-like bonds. Similar bonds are also formed in vitro; for example, Insulin readily combines with the thiocyanate anion [6].
Organic anions and cations combine with proteins through the same type of electrovalent bond. Studying the Binding of Proteins with colored ions offers certain methodological advantages. While the combination with colorless ions can only be investigated using very laborious Analytical Methods, the combination of proteins with Dyes can be studied spectroscopically, since The process of dye ion binding is accompanied by A change in color and absorption spectrum. This approach has been used to quantitatively study the binding of proteins to methyl orange and other similar dyes [8, 9], as well as to nitrophenols [10]. By dialyzing serum albumin against methyl orange, it was established that the maximum number of dye molecules bound per protein molecule is 22. Methyl orange is an acidic azo dye:
Class="center">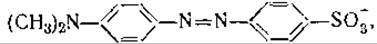
whose sulfonate anion binds to the cationic groups of the protein, specifically to the ε-amino groups of Lysine [9]. At pH >12, the basic groups of lysine lose their positive charge (see p. 78), and The amount of bound dye decreases. The color of a methyl orange solution at constant pH changes upon The addition of protein because the protein, by combining with the dye anions, thereby disrupts the equilibrium between the anions and undissociated dye molecules [9]. Thermodynamic analysis shows that The change in Free energy of the reversible reaction

is ∆F = —6411 cal per 1 mol of dye at 25° [8, 11]. It was also established that ∆H is —2100 cal/mol [11]. Using a similar analysis, it was possible to show that 1 molecule of serum albumin combines with only 6 molecules of o-nitrophenol, whereas the reaction with m-nitrophenol involves the combination of 1 albumin molecule with 24 molecules, and with p-nitrophenol — with 25 molecules [10]. These data clearly indicate that the Nature of the binding is determined by THE POSITION OF the reacting groups¹. Proteins can form compounds not only with aromatic dyes, but also with such simple aliphatic anions as butyrate, caproate, and caprylate anions. This was established by Electrophoresis and is further supported by the fact that fatty acid anions protect proteins denatured by heat or other means against coagulation [13].
Of considerable interest is the fact that methyl orange, which readily combines with serum albumin, does not form compounds with γ-globulin, insulin, Pepsin, and Trypsin [11]. Lactoglobulin, on the other hand, is capable of binding small amounts of methyl orange [11]. Such a difference in The behavior of individual proteins indicates that The surface of their globular molecules is formed by different molecular groups.
Denatured egg albumin combines very tightly with the azo dye Congo red, which protects egg albumin from heat coagulation [14]. The dye anion binds so firmly to the denatured protein that it continues to exist as a red-colored anion even at pH 2, whereas free Congo red anions turn into Congo blue already at pH values below 3–4. In salt-free solutions, Congo red forms precipitates with proteins [15]. Congo red is also capable of binding to an insoluble protein — amyloid — which accumulates in the Liver, Spleen, and other Organs in certain chronic inflammations. This reaction is used for the Diagnosis of amyloidosis, since intravenously administered dye, being bound by amyloid, disappears from the Blood of patients suffering from amyloidosis faster than from the blood of other patients. Staining amyloid with Congo red is also of special interest because the protein–dye complex exhibits birefringence, whereas amyloid itself does not possess this property [16].
¹ The combination of proteins with triphenylmethane dyes was studied in detail by A. D. Brown and his coworkers (A. D. Brown, Dissertation, Leningrad, 1949; A. D. Brown, Biochemistry, 13, 409, 1948; DAN USSR, 62, 263, 1948; 68, 757, 1949; Biochemistry, 16, 399, 1951). Their work established that the ability of many proteins to decolorize triphenylmethane dyes (malachite green, brilliant green, and others) is due to the formation of compounds between these dyes and proteins, with denatured proteins possessing a greater binding capacity for these dyes than native ones. The dyes attach to The sulfhydryl groups of proteins. — Ed. note.
A multitude of studies have been carried out on protein compounds with anionic detergents. The latter are long-chain alkyl sulfonic acids (RSO3H) or alkyl sulfuric acid esters (ROSO3H). In most of these works, sodium dodecyl sulfate (C12H25∙ OSO3Na) was used as the anionic detergent. At pH values below the isoelectric point of the protein, anionic detergents form insoluble precipitates with proteins. Since the isoelectric point of most proteins lies around pH 5–6, precipitation by anionic detergents occurs in a clearly acidic reaction, and, obviously, the detergent anions combine with the cationic groups of the protein [17]. β-Lactoglobulin combines with two molecules of dodecyl sulfate [18], forming a crystalline compound. However, if the protein is mixed with a large excess of detergent, each protein molecule will combine with a very large number of detergent anions. For example, 100 g of gelatin bind more than 1000 mM of dodecyl sulfate, although this amount of gelatin contains only 90 meq of cationic groups [19]. To explain such an unexpectedly high detergent-to-protein ratio, it has been suggested that not individual molecules, but multimolecular detergent micelles combine with the protein; it can also be assumed that, alongside the formation of salt-like bonds, the detergent is bound to the protein molecule by forces acting between the hydrocarbon chains of the detergent and the hydrophobic groups of the protein [21]. The formation of insoluble protein-anionic detergent complexes has also been observed in monomolecular films at the Water–air interface [22], this reaction being accompanied by Protein Denaturation. When a 4% egg albumin solution was mixed with a 5% detergent solution in the presence of ammonium sulfate, the formation of insoluble threads was observed [23]. The precipitates probably consist of alternating layers of protein and detergent [24]. The protein–detergent complex is soluble in an excess of detergent, which is apparently associated with the formation of a complex centered on the protein molecule and having a surface formed by the anionic groups of the detergent [25]. Soluble protein–detergent compounds are also formed in alkaline solutions [17, 25]. Their presence can be detected electrophoretically.
Similar compounds are formed between proteins and acidic azoproteins. If the reaction takes place in the interisoelectric zone, i.e., in the pH region between the isoelectric points of the protein and the azoprotein, the resulting complex precipitates [26]. Acidic azoproteins are prepared by coupling a protein with diazotized aminobenzenesulfonic acids; they contain acidic sulfo groups and exist as anions at pH > 2. Protein–azoprotein precipitates dissolve at pH > 8, since at this pH value both the protein and the azoprotein are anions. Protein–azoprotein precipitates are also soluble in an excess of azoprotein, analogously to how protein–detergent precipitates dissolve in an excess of detergent.
In addition to the aforementioned macromolecular anions, proteins also form compounds with polyacid anions, such as the acids contained in pectin or gum arabic. These compounds also precipitate in the interisoelectric zone and dissolve in an excess of the anion [27]. The precipitates formed upon the combination of proteins with these fibrillar anions have a loose gel-like Structure and represent microscopic droplets rather than a solid phase. This form of precipitation, termed coacervation [28], is caused by the immobilization of large amounts of water between the fibrillar polyacid anions.
The reactions occurring between proteins and macromolecular anions are of particular importance because they can serve as models for the combination of proteins with Nucleic Acids, which are also high-molecular-weight anions. The reactions of nucleic acids with proteins will be discussed below (see Chapter XI). Anticipating, however, we can say that nucleic acids behave similarly to the anions considered above, combining with proteins via salt-like bonds and forming precipitates in the interisoelectric zone [29, 30]. From what has been said, it is clear that anions should most readily combine with proteins possessing basic properties. Lysozyme, a basic protein whose isoelectric point lies at pH 10.5–11.0, combines in neutral solutions with nucleic acids, as well as with anionic detergents and methyl orange [31].
The combination of proteins with organic cations has been studied much less thoroughly than the combination with anions. Strongly alkaline protamines yield precipitates with globulins and with denatured (but not native) albumins. These precipitates form in the interisoelectric zone, i.e., in an alkaline reaction, and dissolve upon acidification [32]. They are also soluble in concentrated solutions of neutral salts. This latter phenomenon is due to the fact that salt ions, successfully competing with the ionic groups of protamine for combination with the ionized groups of the protein, break the established protein–protamine bonds [33].
In recent years, cationic detergents (invert soaps) possessing disinfectant properties have been prepared synthetically. These substances combine with proteins in the interisoelectric zone, i.e., in alkaline solutions. Most cationic detergents have the structure  where
 is a halide ion, and R represents various aliphatic or cyclic groups. Zephiran (zephirol), one of the cationic detergents, is dodecylbenzyldimethylammonium chloride (or dodecyltrimethylammonium chloride); in alkaline solutions, it forms precipitates with proteins that dissolve in an acidic reaction when the negative COO groups of the protein lose their charge [35, 36]. These precipitates are also soluble in an excess of cationic detergent [37]. An analysis of precipitates obtained by the action of desogen (tolyldodecyltrimethylammonium methosulfate) on Hemoglobin showed that a hemoglobin molecule binds over 300 detergent cations; since a hemoglobin molecule contains only 65 anionic groups, it is believed that cationic detergent micelles attach to the protein molecule [38].
There is still insufficient evidence to assert that the disinfectant action of cationic detergents is due precisely to their binding of bacterial proteins. It is known that cationic detergents also combine with neutral Polysaccharides, and therefore their binding of polysaccharides comprising the bacterial capsules may also play a significant role in The Mechanism of disinfectant action.
At present, there is no doubt that anionic and cationic detergents are attracted to proteins via the ionized groups of the protein molecules; however, it is also highly probable that the nonpolar hydrocarbon chains of the detergents participate in the formation of these compounds. The nonpolar hydrocarbon group apparently combines with the nonpolar groups of the protein, i.e., with the aliphatic chains of Alanine, valine, leucine, and isoleucine, with the benzyl group of phenylalanine, and with the CH2 groups of the Proline pyrrolidine ring. By means of these nonpolar groupings, proteins combine with fats and Fatty acids [39], as well as with simple Hydrocarbons. For example, it was established that a 2% solution of edestin in 10% sodium chloride is capable of keeping in solution 5,000 molecules of pentane per protein molecule [40]. The adsorption of low-molecular-weight polar compounds (e.g., carbon tetrachloride) by the intestinal wall may be due to the same phenomenon — the loose binding of these compounds by proteins.
Hydroxyl, sulfhydryl, amide, and other deionized polar or polarizable groups of protein molecules combine with polar or ionic groups of other molecules via electrostatic forces. Many drugs, including sulfonamides, also attach to protein molecules through these same bonds. The free energy change upon the combination of proteins with sulfonamides is ∆F = 4,000–5,000 cal/mol [41]. The spatial arrangement of the polar groupings entering into the bond exerts a major influence on bond strength. The better the two reacting partners are "fitted" to each other, the smaller the intermolecular distance between them will be, and the stronger the mutual attraction between their ionic or polar groups will prove to be [4]. The mutual attraction between Antigens and their specific Antibodies is due precisely to this type of bond — the mutual attraction of complementary surfaces (see Chapter XIV).
Competitive inhibition is due to the same effect, namely, the competition of structurally similar molecules for binding to the exact same part of the protein molecule whose surface shape is complementary to theirs. The Introduction/43.html">Action of Certain antimetabolites can be explained on this basis. A good example of this kind is the competition of p-aminobenzoic acid with sulfonamides. The reason for this competition lies in the analogous Spatial Structure of both named compounds:

Similar competition between substrates and inhibitors (in enzymatic reactions) and between antigens and haptens will be discussed in Chapters XII and XIV.
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.