Biochemistry of Amino Acids - A. Majster 1961
General Biochemistry and Physiology of Amino Acid Metabolism
Synthesis of Peptide Bonds
Synthesis of Glutamine
In 1935, Krebs first observed glutamine synthesis in experiments with tissue slices [540]. The resulting glutamine was isolated as the hydrochloride [541]. Krebs noted that glutamine synthesis in guinea pig tissue preparations is inhibited under anaerobic conditions and upon The addition of cyanide, leading him to conclude that this synthesis depends on energy-yielding reactions [540]. In later work with Cell-free systems, Bücher and Leuthardt [542], Speck [543, 544], and Elliott [545–547] found that adenosine triphosphate can serve as the energy source for glutamine synthesis. The enzyme system responsible for glutamine synthesis has been found in the Liver, Brain, and certain other Tissues of various animal species, as well as in Bacteria and plants [62, 542–556]; it catalyzes the following reaction:
Class="center">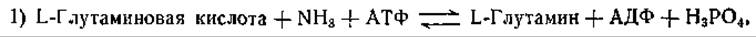
as well as a similar reaction in which ammonia is replaced by hydroxylamine:
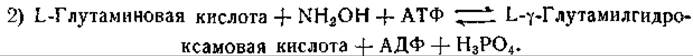
Both reaction (1) and reaction (2) require the presence of magnesium or manganese ions; stoichiometric amounts of ATP are utilized in these reactions. Furthermore, the glutamine-synthesizing enzyme system catalyzes the following transfer reaction:
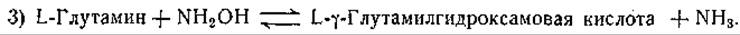
This reaction requires the presence of magnesium or manganese ions and catalytic amounts of adenosine triphosphate and inorganic phosphate (adenosine triphosphate is less effective than a mixture of adenosine diphosphate and inorganic phosphate).
L-Glutamic acid can be replaced by D-glutamic acid [557] and certain racemic derivatives of glutamic acid (e.g., α-methylglutamic acid [558–560] or β-methylglutamic acid [560]); generally, reaction (1) proceeds more slowly with these derivatives than reaction (2). The transfer reaction (3) can take place to some extent in a system containing α-methylglutamine, whereas other glutamine analogs show no appreciable activity. In addition to ammonia and hydroxylamine, hydrazine, methylamine, and Glycine ethyl ester can participate in the synthesis reaction, yielding the corresponding γ-glutamyl derivatives.
It has been established that the glutamine synthesis reaction is reversible. Based on the Equilibrium Constant of reaction (1), it has been calculated [561] that under standard conditions, the difference between the standard free energies of glutamine Hydrolysis and ATP hydrolysis is 4,300 cal. Assuming that the Free energy of glutamine hydrolysis is –3,500 cal (i.e., approximately the same as for asparagine hydrolysis), the Standard Free Energy of ATP should be close to –7,800 cal. This value is somewhat lower than that obtained in earlier determinations, i.e., –10,500 [562, 563], but is in good agreement with values obtained later using A wide variety of Methods [535, 564–566].
Although glutamine synthesis is a reversible reaction, studies using C14-glutamic acid have shown that free glutamic acid is not an obligatory intermediate in the transfer reaction (3). In other words, The conversion of glutamine to γ-glutamylhydroxamic acid does not involve The formation of glutamic acid via the reversal of synthesis, but likely proceeds through the formation of an intermediate compound that reacts with hydroxylamine [560]. Enzyme preparations that carry out glutamine synthesis catalyze yet another reaction—the arsenolysis of glutamine, i.e., the conversion of glutamine to glutamate and ammonia in the presence of arsenate, Mg++ (or Mn++), and adenosine diphosphate [561]. Experimental data indicate that the synthesis, transfer, and arsenolysis reactions are catalyzed by the same enzyme. This Conclusion is supported by the fact that during Enzyme Purification, a parallel increase in activity is observed for all three reactions, and upon ultracentrifugation of the preparations, these activities sediment with the same monodisperse fraction. Moreover, these reactions were found to require approximately the same NUCLEOTIDES and Metal Ions. Certain differences have been described in the effects of metal ions, activators (e.g., β-mercaptoethanol, Cysteine), and inhibitors (e.g., fluoride) on the synthesis and transfer reactions, but this cannot serve as proof that different Enzymes are involved.
No other Cofactors or free intermediates have been detected. Neither γ-glutamyl phosphate nor amidophosphoric acid (O = P(OH)2NH2) exhibits activity [544, 567]. According to A number of studies, enzyme preparations catalyzing glutamine synthesis mediate the exchange of P32-phosphate among ATP, ADP, and inorganic phosphate [561, 568, 569]. Interestingly, the phosphate exchange reaction requires the presence of L-glutamate and ammonia [707]. There are reports that similar reactions are catalyzed by enzymes involved in Glutathione synthesis (p. 268). It has also been demonstrated that glutamine synthesis [reaction (1)] is coupled with The transfer of an ω-oxygen atom (labeled with O18) from glutamic acid to inorganic phosphate [570–572, 708]. Although these data point to the formation of a γ-glutamyl phosphate bond, other interpretations cannot be ruled out. If the synthesis and transfer reactions are indeed catalyzed by the same enzyme, any proposed mechanism must obviously account for the requirement of ADP and phosphate in the transfer reaction. Such a mechanism must also be consistent with the narrower substrate Specificity of the transfer reaction compared to the synthesis reaction.
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.