Biochemistry and Molecular Biology - Belyasova N.A. 2002
Fundamentals of Genetic Engineering
Construction and Analysis of Genomic Libraries
Introduction of a Gene into a Vector
A Gene obtained by one method or another can direct the synthesis of its corresponding product only within a Cell, provided that it is expressed. Furthermore, the gene must be capable of Replication so that all Cells in a population contain it and produce the required amount of the product. All of these conditions—gene delivery into cells, their replication, METABOLISM/31.html">Transcription, and Translation—are mediated by vector DNAs (vectors).
Vectors are defined as small, autonomously replicating DNA molecules—specifically Plasmids, phage DNAs, or other Viruses, or their modifications—that ensure penetration into The Cell and the stable inheritance of foreign DNA (genes). Vector replicons must meet several requirements: they must contain a replication ori and replicate autonomously; be stably inherited by the host cell; be present in high copy number within the cell; possess sufficient capacity to allow the cloning of large genes; contain convenient restriction sites; carry markers for the direct Selection of cells that have taken up the cloned DNA segment and the vector itself; and have a broad host range, among other properties.
Because plasmids, like the viruses used to construct cloning vectors, are inherently specific to the species of organisms in which they can replicate, vector design must take into account the intended host cells for cloning. Among the numerous vector-host systems developed to date, the most widely used are those employing the bacterium E. coli as the host, with plasmids or Bacteriophages of Escherichia coli serving as the vectors. It is worth noting that early concerns among scientists regarding the unpredictable outcomes of eukaryotic Gene cloning spurred the search for and creation of attenuated host bacterial strains. Specifically, "safe" E. coli K12 strains were developed, featuring several characteristics that preclude "escape" from the laboratory: dependence on specific growth factors absent in natural ecological niches, and a fragile Cell wall sensitive to slightly hypotonic media, among others.
Plasmid Vectors. A large number of vectors based on plasmid replicons have been engineered for E. coli, among which derivatives of the ColE1 plasmid, particularly pBR322 (Fig. 20.4), have gained special prominence. This vector was constructed by combining in vivo Genetic Methods with Recombinant DNA technology.
Plasmid pBR322 is 4362 bp in length, and its complete nucleotide sequence has been established. The vector contains genes conferring resistance to two Antibiotics—ampicillin and tetracycline—as well as 12 unique recognition sites for Restriction Endonucleases (each of the 12 restriction Enzymes cleaves the molecule at only one site).
The advantages of this vector are as follows. First, it can be present in cells in a high copy number per chromosome. Second, it contains two selectable markers (ampicillin and tetracycline resistance), with restriction sites for several enzymes located within the genes determining Antibiotic Resistance. This feature means that if a foreign DNA fragment is inserted into a site located inside a resistance gene, that gene is inactivated, allowing cells that have inherited the plasmid with the cloned DNA fragment to be identified by the loss of resistance to the corresponding antibiotic. For example, if the restriction enzyme PstI is used to insert the DNA fragment, the integrity of the gene responsible for ampicillin resistance is disrupted. However, tetracycline resistance remains intact, enabling cells containing such vectors to be selected on media containing tetracycline and subsequently screened for sensitivity to the second antibiotic to identify those harboring the cloned fragment.
Class="center">
Fig. 20.4. Restriction map of plasmid pBR322. Shown are: THE ORIGIN OF replication (4362/1); the genes for ampicillin resistance (Amp-r) and tetracycline resistance (Tet-r); and restriction sites for several endonucleases.
In Introduction/32.html">Genetic Engineering, this technique is referred to as "insertional inactivation of a marker."
Other strategies exist for selecting cells that have taken up vectors containing inserted DNA. One such approach relies on the ability of the N-terminal portion of ß-galactosidase to Complement a specific mutant ß-galactosidase in the bacterial cell. The Procedure is as follows. A segment of the E. coli lac Operon, including the promoter, operator, and 5'-coding region of the lacZ gene (which encodes the N-terminal part of ß-galactosidase; Figs. 3–5), is introduced into the vector. A polylinker is inserted into this region without disrupting either the reading frame or The activity of the N-terminal ß-galactosidase fragment. The polylinker is an artificially synthesized sequence containing multiple restriction sites for various Nucleases. If the polylinker lacks an insert, such a vector genome directs the Synthesis of the N-terminal fragment of ß-galactosidase, which, together with the C-terminal fragment produced by a special E. coli strain, forms active ß-galactosidase. This enzyme produces a blue coloration in cells grown on media containing the chromogenic substrate Xgal and an inducer. If foreign DNA is inserted into the polylinker, complementation is disrupted, and cells taking up the recombinant DNA form uncolored colonies.
Vectors constructed from plasmid replicons have certain drawbacks, the primary one being a decrease in copy number per cell as the size of the hybrid plasmid increases. As a consequence, the cloning of DNA fragments exceeding 10 kb becomes inefficient. To clone such large DNA fragments, phage vectors, cosmids, and phasmids are employed.
Phage vectors. When using phage vectors, the viable product containing the recombinant DNA is a population of phage particles rather than a population of cells, as is the case with plasmid vectors. Phage vectors are more efficient than plasmids for cloning large inserts. The most widespread vectors for E. coli are those derived from bacteriophages λ and M13.
The Genome of temperate phage λ consists of a double-stranded DNA molecule of 48.5 kb, packaged into the phage HEAD as a linear molecule with single-stranded complementary ends (sticky ends). Upon entering the host cell, the sticky ends pair, and the molecule circularizes and is covalently sealed by DNA ligase. The sites of sticky-end pairing are designated as cos-sites; they participate in the generation of phage genomes during rolling-circle replication (Chapter 1). The λ prophage in lysogenic cells exists in a state integrated with the nucleoid (the mechanism and features of this process are described in Chapter 2).
Certain Features of the λ phage genome are crucial for vector design. First, the entire central region (more than 1/3 of the genome) is non-essential for the lytic cycle and is required solely for establishing and maintaining Lysogeny. Consequently, it can be replaced by foreign DNA while the phage retains its ability to lyse cells. Second, successful packaging of DNA into phage heads requires the molecule to be between 38 kb and 52 kb in length.
A wide variety of vectors based on phage λ have been constructed to date. Typical Examples contain EcoRI restriction sites flanking a region of the genome that is non-essential for the lytic cycle (Fig. 20.5). Digestion of such vector DNA with EcoRI yields three fragments, from which the terminal fragments (containing genes required for the lytic cycle) can be isolated due to their relatively large size. These fragments are mixed with foreign DNA digested with EcoRI, yielding hybrid molecules in which the central region is replaced by the insert fragment (Fig. 20.5). The resulting hybrid molecules are then packaged into λ phage heads in vitro. This is accomplished using E. coli cell cultures infected with mutant λ phage strains—one carrying a defect in a gene responsible for packaging DNA into the head, and the other defective in the Synthesis of specific head Proteins. Such phages cannot complete the lytic cycle, but they drive the intracellular accumulation of high levels of the intermediates required for phage particle assembly: empty heads, tails, and essential assembly enzymes. When extracts of these cells are mixed with vector DNA containing inserts of a specific size, packaging into phage heads occurs, yielding mature phage particles. In the next step, sensitive cells are infected with these particles to propagate progeny phages carrying the cloned DNAs. Fragments up to 15 kb in length can be cloned using λ phage-based vectors.

Fig. 20.5. Insertion of genes into λ phage-based vectors.
Another category of phage vectors for E. coli is based on the M13 phage genome. This filamentous "male-specific" phage (which adsorbs to F-pili) contains single-stranded DNA. When the phage DNA enters an E. coli cell, it replicates via double-stranded ("+"/"-") intermediates, whose "+" strands are subsequently repackaged to yield numerous progeny phage particles. The double-stranded intermediate (the replicative form, RF) accumulates in the cells at 100 to 200 copies per cell. It is isolated and used as a cloning vector. A notable feature of M13 is that it does not kill the host cells, but merely slows their division. Phage particles are continuously secreted into the culture medium, and their titer can reach 1012 per ml. On a lawn of sensitive Bacteria, the phage produces turbid plaques.
Polylinkers are incorporated into the phage DNA to facilitate the introduction of foreign DNA. When a heterologous sequence is inserted into the M13 RF DNA, only one of the strands of this insert is packaged into the phage particles (Fig. 20.6). Single-stranded DNA molecules are generally unsuitable for vector construction because they cannot be cleaved with commonly used restriction enzymes. By cloning a fragment in M13 in both orientations, large quantities of each individual strand can be obtained.
To facilitate the selection of recombinant forms (phages whose genomes harbor an inserted foreign DNA fragment), vectors incorporate a segment of the E. coli lac operon into a non-coding region, which directs the complementation of mutant ß-galactosidase, along with a polylinker. When the polylinker lacks an insert, phage particles grown on a special mutant E. coli strain in the presence of an inducer and a chromogenic substrate form blue negative plaques. Insertion of a DNA fragment into the polylinker disrupts complementation, leaving the plaques colorless.
An advantage of M13-based phage vectors is their ability to accommodate very large inserts, since packaging in this system is not strictly dependent on the overall size of the phage genome. The most important application of M13-derived vectors is the generation of single-stranded DNA templates for Sanger sequencing. Furthermore, single-stranded DNAs serve as ideal templates for Site-Directed Mutagenesis.
An Analysis of the points discussed above reveals distinct advantages for both plasmid and phage vectors, which inspired The Development of vectors combining The properties of both. These are the so-called plasmid-phage vectors, a group that includes cosmids and phasmids.
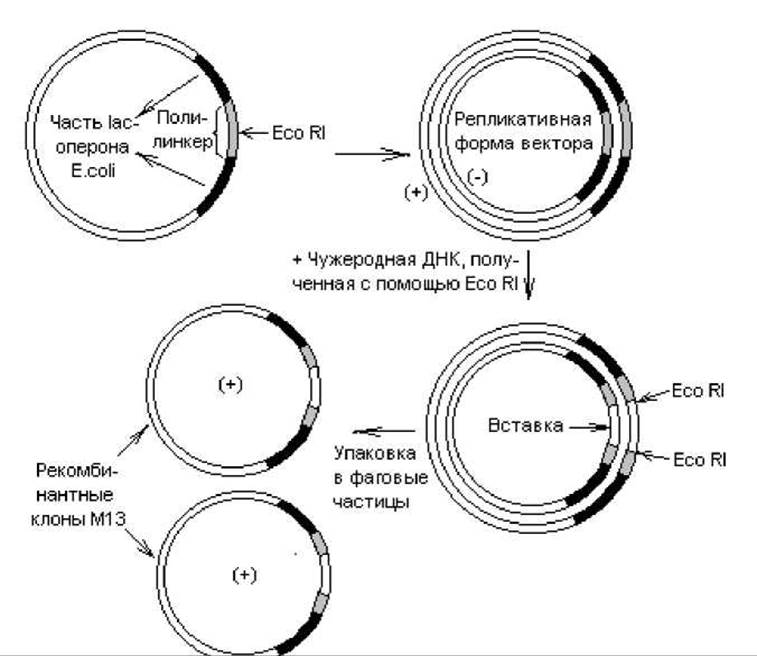
Fig. 20.6. Insertion of DNA fragments into M13 phage-based vectors.
Cosmids. Cosmids represent a type of hybrid vector that replicates via a plasmid mechanism while retaining The ability to be packaged in vitro into λ phage capsids. In other words, cosmids are plasmids that contain the cos-site (sticky ends) of λ phage DNA. Because of these cos-sites, these vectors can be introduced into cells not by transformation, but via conventional infection, which increases the efficiency of recombinant cell recovery by 100-fold or more. Cosmid vectors can accommodate DNA fragments ranging from 33 to 49 kb in size, making them ideally suited for cloning large eukaryotic genes—a capability of particular importance for constructing eukaryotic Genomic Libraries.
An example of a cosmid vector is the plasmid pBR322, which has phage λ cos-sites cloned into its ampicillin resistance gene. If such a vector is cleaved with a restriction endonuclease and mixed with foreign DNA fragments obtained by digesting a genome with the same restriction enzyme, a mixture of concatemers may form.
Concatemers are long molecules in which phage λ genomes (or the DNA substituting them) repeat multiple times and are separated from each other by cos-sites (Fig. 20.7). When these concatemers are mixed with phage λ DNA-packaging proteins, they are cleaved at the cos-sites, and the DNA is packaged into the capsid. For this to occur, the distance between two adjacent cos-sites must be 38–52 kb.
As with λ vectors, the mixture of concatemers may include vector molecules without inserts, as well as those with multiple repeating inserts. Following cell infection, the recombinant DNA is maintained within them as a plasmid, in this case conferring resistance to tetracycline.

Fig. 20.7. Using cosmid Vectors for Cloning.
Phasmids. These are also hybrid vectors capable of developing both as a phage and as a plasmid, since they contain all the genes necessary for the lytic cycle as well as those required for plasmid replication. The cloning capacity of phasmids is smaller than that of cosmids and comparable to that of phage vectors. The advantage of phasmids is that their DNA size is too small for a monomer to be packaged into a phage λ capsid, yet too large for a vector dimer to be packaged. Therefore, negative colonies can only be formed by recombinant phasmids, as their sizes match the capacity of the phage λ head.
The insertion of a foreign DNA fragment into a phasmid is carried out similarly to the previously described examples for other vectors, most frequently via restriction sites. Subsequently, the hybrid phasmids are packaged into capsids in vitro, as described above. Upon infection of sensitive cells, phasmids drive the lytic cycle and form plaques on a lawn of the test culture. However, if the vector contains the $d$ gene encoding The Structure of the repressor protein, the phasmid replicates as a plasmid rather than a phage. Often, mutant $d$ genes are employed within phasmids, determining the structure of a Temperature-sensitive repressor protein that is inactivated at elevated temperatures. In this case, the phasmid behaves as a plasmid at low temperatures, but upon raising the temperature by a few degrees, it is induced into the lytic cycle. This property of phasmids proves very useful in many Applications.
Certain bacteriophages exhibit phasmid properties, such as phage P1, which in the prophage state does not integrate into the chromosome but is maintained as a plasmid. The phage P1clr100 mutant can be induced into the lytic cycle at temperatures above 32 °C, meaning it behaves as a typical phasmid.
The vector types used for gene cloning in E. coli cells have been characterized above. For other prokaryotic species, numerous diverse vector molecules have also been constructed, among which so-called "shuttle vectors" are particularly noteworthy. Their distinct feature is the ability to replicate in different host cells, which is ensured by introducing additional origins of replication (ori) into the vector, along with genes required for replication that are not provided by the host cells. Some shuttle vectors can be maintained in various Prokaryotic Cells, while others function in certain PROKARYOTES AND EUKARYOTES (Yeasts, plants, animals). The Use of shuttle vectors offers a distinct convenience for gene cloning and the analysis of their products, as it allows the same genes to replicate and express in different organisms.
One example of constructing shuttle vectors is the combination of a portion of the 2 µm (two-micron) Yeast plasmid from Saccharomyces cerevisiae with the plasmid pBR322 containing the yeast HIS3 gene (which encodes one of the enzymes for Histidine Biosynthesis). It turned out that the HIS3 gene is also expressed in bacterial cells because it contains a region homologous to the corresponding E. coli promoter. Such a vector replicates in both S. cerevisiae yeast cells and E. coli bacteria, enabling the direct selection of cells that have taken it up by using histidine-dependent strains on a synthetic medium lacking this amino acid.
The basis for vectors designed to clone animal genes is most frequently the simian virus 40 (SV40) genome. The General Principles of vector construction in this case are the same as those for phage λ-based vectors.
For plant cells, which lack endogenous plasmids, vector backbones are frequently derived from plant virus genomes as well as the pTi bacterial plasmid, which mediates The transfer of plasmid DNA segments into the genomes of various dicotyledonous plants and induces crown gall tumor formation. The family of pTi plasmids has been identified in the Gram-negative bacterium Agrobacterium tumefaciens.
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.