Biochemistry and Molecular Biology - Belyasova, N.A. 2002
Molecular Foundations and Mechanisms of Heredity
Maintenance of Genome Stability and Variability
Activity of Mobile Elements
Mobile Genetic Elements include the Mu prophage, Transposons, and IS-elements (Insertion Sequences), which are discrete segments of DNA capable of moving within a single genome or between genomes residing in the same Cell. All mobile elements contain genes that mediate the transposition process, as well as specific inverted repeats at their ends that also participate in mobility.
IS-elements are linear DNA fragments ranging from 0.2 to 2 kb in size, featuring inverted repeats at their extremities (flanked by repeats). There are several types of IS-elements, which differ in their nucleotide sequence, length, the size of their inverted repeats (10–40 bp), transposition frequency (10-4–10-7 per generation), and the length of duplicated target DNA repeats (5–11 bp) generated during transposition. IS-elements do not contain genes determining phenotypically distinct traits; rather, they carry only the information necessary for the transposition process (The Structure of the transposase enzyme). When these elements transpose to a new site, the original IS-element remains in place—meaning that insertion is accompanied by the precise synthesis of a second copy and does not depend on the host's replicative Functions or recombination machinery. Furthermore, no Homology is required between the IS-element and the target site. Different replicons contain varying numbers of IS-element copies: for example, the E. coli nucleoid contains 4–19 copies of IS1, 0–12 copies of IS2, and 1–2 copies of IS4.
Transposons (Tn) are complex mobile structures created on The basis of IS-elements (or their derivatives) that contain genes determining additional functions (other than transposition). All transposons are flanked by terminal repeats. These are often well-known IS-elements, such as IS1, which can repeat at the transposon ends in either direct or inverted (Fig. 2.9) orientation.
As seen in Fig. 2.9, the central region of the transposon (Km) is flanked on both sides by identical IS-elements: IS-L (left) and IS-R (right), which are located in Tn5 in opposite orientations. At the same time, the IS-elements themselves also contain inverted terminal repeats. All the information required for the movement of a complex transposon is contained within its IS-elements—specifically, the same Genetic information that IS-elements use during transposition, namely the genes encoding transposase.
Different mobile elements vary in their degree of Specificity when selecting integration sites within replicons. With high specificity, a transposon utilizes one or a few target DNA sites; with low specificity, it uses multiple preferred sites or practically any site. The probability of transposition depends on The properties of the mobile element, primarily its length: for every 1 kb increase in transposon size, the frequency of movement decreases by half. The transposition frequency for the same mobile element can also vary depending on The Nature of the donor and recipient replicons. For instance, certain Mutations are known to suppress transposition frequency. Additionally, the movement of mobile elements is influenced by environmental factors such as Temperature, UV irradiation, and chemical agents.
Mechanism of Transposition. To explain The Mechanism of transposition, the subtleties of which remain elusive, several models have been proposed, belonging to two main groups: replicative and conservative. The replicative (cointegrative) model is the most straightforward. According to this model, The First stage involves the fusion of donor and recipient DNA molecules, accompanied by duplication at the sites where the two replicons merge (Fig. 2.10).
Class="center">
Fig. 2.9. STRUCTURE OF THE Tn5 transposon: NK — target replicon DNA; D — duplicated target regions; Km — kanamycin resistance genes. Arrows indicate the directions of terminal repeats within the IS-elements, as well as the orientation of the IS-elements themselves at the transposon ends
At the Second Stage, the replicons separate through reciprocal recombination between identical regions (res sites) within the cointegrate (Fig. 2.10).
The execution of the first stage requires transposase and two inverted terminal repeats. It is believed that transposase specifically recognizes and interacts with these exact regions. Resolving the cointegrate requires another product of the transposon genes—resolvase—which mediates Site-Specific Recombination at the res sites.
During transposition via cointegration, not only the genes belonging to the mobile element itself are involved, but also The Cell's replicative functions. For instance, cointegrates of certain transposons have been shown to dissociate only in RecA+ Cells (which contain the RecA protein); in other words, the resolution of these cointegrates proceeds with the participation of the Homologous Recombination system.
The conservative (simple, non-replicative) model of transposition involves the excision of the mobile element from the donor molecule and its insertion into the recipient molecule, meaning that the mobile element itself is not duplicated. Even in this case, however, the hallmark feature of transposition is preserved: duplicated repeats arise at the target site (Fig. 2.11). According to the conservative model, transposase catalyzes staggered double-stranded breaks in the recipient DNA, similar to those produced by restriction Enzymes. Transposases likely make incisions at the ends of the transposon and join them to the ends of the breaks in the target DNA. This forms single-stranded gaps that are subsequently filled in by the cell's repair systems. As a result, short identical repeats of the target DNA region are consistently generated at the ends of the mobile elements (Fig. 2.11). Some mobile elements, such as the Mu bacteriophage, can participate in both types of transposition: integrative and conservative.
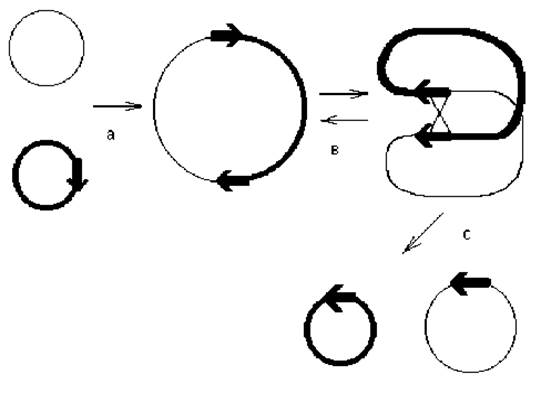
Fig. 2.10. Mechanism of replicative transposition: a — Formation of the cointegrate; b — reciprocal recombination between res sites; c — resolution of the cointegrate. Transposons are indicated by arrows
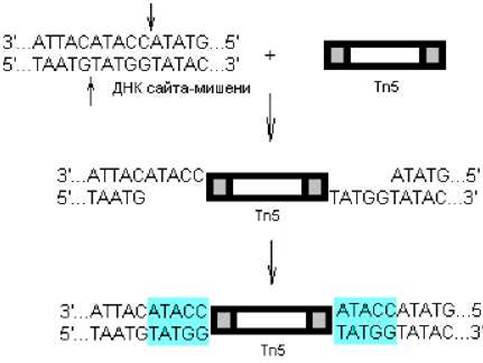
Fig. 2.11. Formation of duplicated repeats in the target DNA during transposition: arrows indicate the sites of covalent bond Cleavage in the DNA resulting from the action of transposase on the target replicon
The excision of transposons from DNA most frequently occurs as a result of homologous recombination between copies of the target site.
The movement of mobile genetic elements within a single replicon can lead to deletions and inversions, while intermolecular transposition may give rise to various other mutations. In general, mobile elements induce all types of chromosomal rearrangements: replicon fusion and dissociation, translocations, deletions, inversions, and duplications. Frequently, the insertion of a mobile element into a regulatory or coding region results in decreased expression of the affected Gene. In some cases, the opposite occurs: a promoter located within the transposon itself drives the expression of a neighboring gene that was previously silent. Alongside Plasmids and phages, mobile elements transfer genes between different organisms and make a significant contribution to their genetic Variability.
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.