Review of Medical Physiology - William F. Ganong 2002
Physiology of Nerve and Muscle Cells
Excitable Tissue: Muscle
Skeletal Muscle: Energy Sources and Metabolism
Muscle contraction requires energy, which is why Muscles are often described as "machines for converting chemical energy into mechanical work." The immediate source of this energy is high-energy organic phosphate compounds stored in Muscle tissue. These substances are produced through carbohydrate and Lipid METABOLISM. The Hydrolysis of ATP, which supplies the energy required for muscle contraction, was discussed above.
Phosphorylcreatine
ATP is generated through the reverse synthesis from ADP, whereby a single phosphate group is added to an ADP molecule. The energy required to drive this endothermic reaction is derived, in part, from The breakdown of glucose into CO2 and H2O. However, muscle tissue contains another high-energy phosphate compound that serves as an alternative short-term energy source for this reaction: phosphorylcreatine (see Figs. 17-21). It breaks down into creatine and phosphate groups, releasing a significant amount of energy. At rest, phosphate groups are attached to creatine within the Cell/35.html">Mitochondria, thereby replenishing phosphorylcreatine reserves. During intense physical exertion, phosphorylcreatine undergoes hydrolysis at the junctions between Myosin heads and Actin, releasing a phosphate group from ATP and generating the energy necessary to sustain continuous muscle contraction.
Class="center">Table 3-4. Isoforms of Myofibrillar Proteins in Adult Rats12

1 Modified from Pette D, Staroń RS: The molecular diversity of mammalian muscle fibers. News Physiol Sci 1993;8:153.
2 Abbreviations used: heavy chain isoforms (HC): HCI - type I; HCII - type II; HCßcard, HCoccard - cardiac; HCIton - tonic; HCeom - extraocular; HCsf - superfasth; Hemb - embryonic; HCneo - neonatal. Troponin subunits (TN): s - slow; f - fast; TN-T - Tropomyosin-binding; TN-I - inhibitory; TN-C - Ca2+-binding.
Breakdown of Introduction/36.html">CARBOHYDRATES and Lipids
During periods of rest and light physical activity, muscles store lipids in the form of free Fatty acids, which serve as an energy source. As exertion increases, lipid metabolism can no longer supply energy quickly enough to support muscle contraction, making carbohydrates the primary energy component for muscles. Consequently, during physical activity, a substantial portion of the energy required for the resynthesis of phosphorylcreatine and ATP is derived from glucose breakdown. The main Metabolic pathways of glucose breakdown are reviewed in Chapter 17. Here, it is sufficient to recall that Blood glucose enters Cells, where complex biochemical reactions ultimately break it down into Pyruvate. Another source of glucose, and consequently pyruvate, within cells is Glycogen—a carbohydrate polymer stored primarily in the Liver. With an adequate supply of O2, pyruvate enters The Citric Acid Cycle and is metabolized through this cycle and the respiratory enzyme chain into CO2 and H2O. This process is known as aerobic Glycolysis. The breakdown of glucose or glycogen to CO2 and H2O releases a large amount of energy, which is sufficient to generate substantial quantities of ATP from ADP. If O2 is available in sufficient quantities, the pyruvate derived from glucose is not incorporated into The Tricarboxylic Acid Cycle, but is instead broken down into lactate. This process—anaerobic glycolysis—yields significantly fewer high-energy phosphate compounds, but has the advantage of not requiring O2. The various Chemical Reactions supplying energy to skeletal muscles are illustrated in Fig. 3-11.
The "Oxygen Debt" Mechanism
During physical exertion, Blood Vessels in the muscles dilate and blood flow increases, resulting in a higher supply of O2. Oxygen consumption is proportional to Energy Expenditure, which is fully met by aerobic glycolytic processes. However, during very intense exertion, the aerobic resynthesis of energy reserves cannot keep pace with their depletion. Under these conditions, phosphorylcreatine is utilized for ATP resynthesis. A certain amount of ATP is also produced during the anaerobic breakdown of glucose to lactate. The anaerobic pathway is quite limited because, despite the rapid rate of lactate diffusion into the bloodstream, lactate accumulates rapidly in muscles at concentrations that far exceed the binding capacity of buffer systems. This leads to a sharp drop in environmental pH, which inhibits enzyme systems. Nevertheless, for short periods, anaerobic glucose breakdown can sustain much more intense muscle contraction than aerobic processes. For example, anaerobic breakdown during a 100-meter dash lasting 10 s provides 85% of the energy; during a 2 km run lasting 7 min, it provides 20%; and during a long-distance run lasting about 1 hour, it provides only 5%.
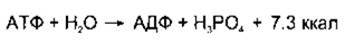
Phosphorylcreatine + ADP ⇄ Creatine + ATP Glucose + 2 ATP (or glycogen + 1 ATP)
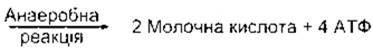
Glucose + 2 ATP (or glycogen + 1 ATP)

Fig. 3-11. Energy released by the hydrolysis of 1 mol of ATP and ATP resynthesis reactions. The amount of ATP generated by The oxidation of 1 mol of free fatty acids (FFAs) is quite large, though it depends on the size of the FFA molecule. For instance, the Complete oxidation of 1 mol of palmitic acid yields 140 mol of ATP.
Following a period of maximal exertion, excess O2 is consumed to clear accumulated lactate, replenish ATP and phosphorylcreatine stores, and restore the small amount of O2 previously carried by Myoglobin. The volume of extra O2 consumed is directly proportional to the extent by which energy demands during exertion exceed the capacity of aerobic systems—in other words, the oxygen debt. Oxygen debt is measured experimentally by determining post-exercise O2 consumption until it returns to a steady baseline level corresponding to basal O2 consumption. Subtracting the basal value from the total consumption yields the oxygen debt figure. This value can be up to six times greater than basal O2 consumption, indicating that an individual is capable of generating muscle force six times more powerful than possible without engaging the oxygen debt mechanism. Oxygen debt is cumulative; it builds up gradually until it reaches a certain ceiling. Naturally, the rate at which it accumulates determines how long a muscle can sustain a specific exertion level. This is why high-intensity efforts are short-lived, whereas moderate efforts can be maintained for quite a long time.
Trained athletes are capable of increasing muscular O2 consumption to a much greater extent than untrained individuals. Furthermore, they utilize free fatty acid (FFA) reserves much more efficiently, allowing them to exert significantly greater muscular force without depleting glycogen stores or increasing lactate production in the muscles. Consequently, they exhibit lower oxygen debt values for any given level of muscular exertion. A few days before major competitions, athletes typically switch to a carbohydrate-rich diet to maximize their glycogen stores, which inherently enhances their endurance.
Rigidity (Stiffening)
When muscle stores of ATP and phosphorylcreatine are completely depleted, muscles enter a state of severe stiffness known as rigor. If this condition occurs As a result of death, it is called rigor mortis. In the state of rigor, all myosin heads remain rigidly bound to actin.
Heat Production in Muscles
According to the Laws of Thermodynamics, the total energy supplied to muscles must equal the energy they expend. Muscle energy is consumed in performing mechanical work, forming high-energy phosphate bonds for future use, and generating heat. The mechanical efficiency of skeletal muscles (The ratio of work performed to energy expended) reaches up to 50% during weight-lifting under isotonic contraction, but drops practically to zero during isometric contraction. Relatively little energy goes into forming phosphate bonds; consequently, a large amount of heat is generated within the muscles. This heat can be measured quite precisely using thermocouples.
Resting heat, produced during rest, is an external manifestation of basic metabolic processes. The additional heat generated During muscle contraction is referred to as initial heat. This heat consists of activation heat—the heat invariably produced whenever a muscle contracts—and shortening heat, which arises only when the muscle length decreases.
Following muscle contraction, excess heat continues to be produced for approximately another 30 minutes. This is recovery heat, which is released as metabolic processes restore the muscle to its pre-contraction state. Recovery heat is roughly equal to initial heat; in other words, the amount of heat generated during recovery equals the amount produced during contraction.
When a muscle restores its initial length after an isotonic contraction, an additional amount of heat, known as relaxation heat, is produced In addition to recovery heat. For the muscle to return to its previous state, work must be performed, and the heat of relaxation is, in fact, a manifestation of this work.
Last update: 10/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.