Biochemistry - The Chemical Reactions of Living Cells, Volume 2 - D. Metzler 1980
How electrons meet oxygen, how ATP is generated in the process, and some related phenomena
Electron Transport Chain and Oxidative Phosphorylation
Thermodynamics and "Reverse Electron Flow"
The ∆G' value for The oxidation of 1 mol of NADH by oxygen (at 1 atm pressure) is —219 kJ (Table 3-7). In Tissues, the O2 pressure is ~10-2 atm, and ∆G' is ~—213 kJ. However, when this reaction is coupled with the synthesis of three molecules of ATP (∆G' = +34.5 kJ∙mol-1), the Free energy change in the overall reaction becomes —110 kJ∙mol-1. This value remains strongly negative. Nevertheless, we must remember that the concentrations of ATP, ADP, and Pi may deviate considerably from the 1:1:1 ratio assumed in Standard Free Energy calculations. An interesting experiment consists in allowing Oxidative Phosphorylation to proceed until Cell/35.html">Mitochondria reach state 4, and then measuring the resulting "mass action ratio" [ATP]/[ADP] ∙ [Pi]. The phosphorylation potential1 expressed in this way (see Supplement 3-A) can reach values of 104 M-1 or higher [73, 76]. As a result, the ∆G value for NADH oxidation in the coupled Electron Transport Chain turns out to be less negative than ∆G0. Indeed, if Electron transport is coupled with the synthesis of three ATP molecules, the system will reach equilibrium at Rp = 106.4 (25°C); the difference between ∆G and ∆G0 is 3RTlnRр = 3∙5.708∙6.4 = 110 kJ∙mol-1.
It is hardly possible to increase Rp enough to achieve true equilibrium between NADH, O2, and the adenylate system; however, equilibrium is attainable within limited segments of the chain. One can even force the electron flow to reverse its direction. Let us consider the passage of electrons along the chain starting from NADH back to fumarate, the oxidized form of the succinate-fumarate couple. The free energy change ∆G' (pH 7) for the oxidation of NADH by fumarate is —67.7 kJ∙mol-1. In uncoupled mitochondria, electron flow will always proceed from NADH to fumarate. However, in tightly coupled mitochondria where ATP is generated at site 1, the overall ∆G' becomes significantly less negative. At Rр = 104 M-1, ∆G' for the coupled process becomes approximately zero (—67.7 + 68 kJ∙mol-1). Electron flow can easily be reversed so that succinate reduces NAD+. Under certain physiological conditions, such ATP-driven reverse electron flow can indeed be observed in living Cells. As we will see later, in some anaerobic Bacteria all NADH is generated through reverse electron flow.
1) This quantity is also referred to as the phosphate potential or phosphorylation potential. However, some define the phosphate potential as the Free energy of ATP formation under specific given conditions, i.e., +34.5 kJ∙mol-1 + RT ln ([ATP]/[ADP]∙[Pi]). Logically, potential should be measured in volts, as in equation (3-64). To avoid confusion, it is best not to use these terms.
Another experimental approach, also based on equilibrium in The electron transport chain, involves measuring the "apparent potential" of a carrier within the chain as a function of ATP, ADP, and Pi concentrations. The apparent potential E is calculated from the lg([oxid.]/[red.]) value according to equation (10-12), where E0' represents the known midpoint potential of the redox couple (Table 3-7), and n is the number of electrons required to reduce one molecule of the carrier:
Class="center">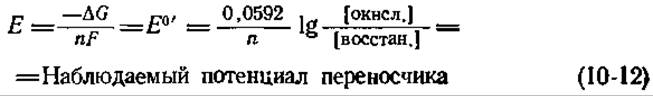
By balancing the system through The addition of a "redox buffer"—a mixture of components of a couple that rapidly equilibrates with the carrier chain (Chapter 3, Section B,1)—one can set E at a predetermined level [73]. For example, a 1:1 mixture of succinate and fumarate fixes E at +0.03 V, whereas a 1:1 ß-hydroxybutyrate—acetoacetate couple fixes E at E0’ = —0.266 V. Let us consider the potential of one of the b-type Cytochromes, designated by Wilson and co-workers as bK. For cytochrome bK, E0’ = 0.030 V. Substituting this value into equation (10-12) and Setting E = —0.266 V (by equilibrating the chain with ß-hydroxybutyrate and acetoacetate), the reader can easily verify that at equilibrium the [oxid.]/[red.] ratio for cytochrome bK will be about 10-5. In other words, in uncoupled mitochondria in the absence of O2, this cytochrome will be almost entirely in its reduced form.
However, if the electron transport chain from ß-hydroxybutyrate to cytochrome bK is tightly coupled to the synthesis of one ATP molecule, the apparent potential of the carrier will be determined not only by the applied potential Ei of the balancing system, but also by the phosphorylation state of the adenylate system [equation (10-13)]:
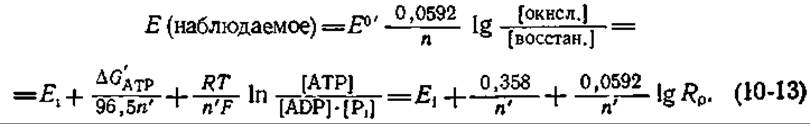
Here ∆G'ATP is the group transfer potential (—∆G' of Hydrolysis) of ATP at pH 7 (Table 3-5), and n' is the number of electrons passing through the chain required for the synthesis of one ATP molecule. Note, however, that in the numerator of the equation, n is the number of electrons required to reduce the carrier; for cytochrome bK, this equals one. Equation (10-13) implies that at a high phosphorylation state, a significant fraction of cytochrome bK remains in the reduced form at equilibrium. Thus, if Rp = 104, E0’ of cytochrome bK = 0.030 V, n' = 2, and the potential E is set using the hydroxybutyrate-acetoacetate couple to —0.25 V, one can calculate from equation (10-13) that the [oxid.]/[red.] ratio for cytochrome bK will be 1.75. If the value of Rp is then varied, the apparent carrier potential will change in accordance with equation (10-13). These changes have been observed experimentally [73]. A tenfold change in Rp alters the apparent potential of cytochrome bK by 0.030 V, exactly as predicted for n = 2. The apparent potential of cytochrome c changes by 0.059 V for each tenfold change in Rp, which is readily predicted given that n' = 2 and that electron transfer to cytochrome c is coupled with the synthesis of two ATP molecules. This provides additional experimental confirmation of a rather fascinating phenomenon. Even with single-electron carriers such as cytochromes, the synthesis of one ATP molecule requires the passage of two electrons down the chain. Furthermore, such experiments lead to the Conclusion that phosphorylation sites are located approximately as shown in Fig. 10-11.
Table 10-6 Electrode potentials of mitochondrial electron carriers and Free Energy Changes associated with electron transporta
|
Electron carrier |
E0' (pH 7) in isolated state |
E0' (pH 7.2) in mitochondria |
∆G (kJ∙mol-1) for transfer of 2e— per O2 molecule at 10-3 atm (carriers at pH 7) |
|
|
Group I |
NADH/NAD+ |
—0.320 |
—213 |
|
|
∼ —0.30 V |
Flavoprotein |
—0.30 |
||
|
Fe—S protein |
∼—0.305 |
|||
|
ß-Hydroxybutyrate-acetoacetate |
—0.266 |
—203 |
||
|
Lactate-Pyruvate |
—0.185 |
—187 |
||
|
Succinate-fumarate |
0.031 |
—146 |
||
|
Group II |
Flavoprotein |
∼—0.045 |
||
|
0 V |
Cytochrome bK |
—0.030 |
||
|
Cu |
0.001 |
|||
|
Fe—S protein |
0.030 |
|||
|
Cytochrome bK |
0.030 |
|||
|
Ubiquinone |
0.10 |
0.045 |
—132 |
|
|
Cytochrome a3+ATP |
0.155 |
|||
|
Group III |
Cytochrome c1 |
0.215 |
||
|
~0.22 V |
Cytochrome c |
0.254 |
0.235 |
—102 |
|
Cytochrome bT+ATP |
0.245 |
|||
|
Cytochrome a |
0.29 |
0.210 |
||
|
Cu |
0.245 |
|||
|
Fe—S protein |
0.28 |
|||
|
Group IV |
Cytochrome a3 |
0.385 |
—77 |
|
|
O2 (10-2 atm) |
0.785 |
0.0 |
||
|
O2 (1 atm) |
0.815 |
a According to Wilson et al. [72, 73].
Another type of experiment is based on equilibrating the electron transport chain with an external redox couple of known potential using uncoupled mitochondria. The E0' value for a given carrier can then be determined from the [oxid.]/[red.] ratio according to equation (10-12). While Changes in the balancing potential E will affect the [oxid.]/[red.] ratio, the E0' value remains constant. For Fe—S Proteins and copper atoms (in proteins) of the electron transport chain, E0' values can be obtained by equilibrating mitochondria and then rapidly freezing them in liquid nitrogen. The [oxid.]/[red.] ratios are subsequently calculated from EPR spectra recorded at 77 K. The results of such measurements, published by Wilson et al. [72–75], are presented in Table 10-6.
Based on their E0' values, mitochondrial carriers are grouped into four isopotential groups with potentials of ∼—0.30, ~0, ~0.22, and ~0.39 V (Table 10-6). When tightly coupled mitochondria enter state 4 (low ADP, high ATP, presence of O2, but low Respiration rate), the apparent potentials shift. For the lowest isopotential group, which includes NAD+/NADH, the potential drops to —0.38 V, corresponding to a more reduced state of the carriers on the substrate side of the first phosphorylation site in Fig. 10-11. Groups 2 and 3 remain near their midpoint potentials of ~—0.05 and +0.26 V. Under these conditions, the potential difference between consecutive carrier groups is ~0.32 V, which is quite sufficient for the synthesis of one ATP molecule per pair of electrons transferred, given an Rр ratio of ≈ 104 M-1 [equation (10-13)].
Two cytochromes behave in a unique manner and are listed twice in Table 10-6. The midpoint potential E0' of cytochrome bT shifts from —0.030 V in the absence of ATP to +0.245 V at high ATP concentrations. On the other hand, the E0’ value for cytochrome a3 drops from +0.385 V to 0.155 V in the presence of ATP. This potential shift suggests that the oxidation of a high-energy reduced form of cytochrome a3 is coupled to ATP synthesis. In the presence of high ATP concentrations, The formation of this intermediate via reduction becomes more difficult (Section D, 9,a). The opposite direction of the E0' shift for cytochrome bT indicates that the oxidized form is the high-energy species in this case [equation (10-11)]. The validity of these Conclusions depends on the precision and reliability with which spectroscopic Methods can measure the [oxid.]/[red.] ratio. Based on these results, it has even been concluded that cytochromes bT and a3 participate directly in oxidative phosphorylation [72–75]. However, this view is far from universally accepted [77].
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.