Biochemistry - The Chemical Reactions of Living Cells, Volume 2 - D. Metzler 1980
Organization of Metabolism: Catabolic Pathways
Tricarboxylic Acid Cycle
Synthesis of the Regenerating Substrate Oxaloacetate
The primary substrate of The Tricarboxylic Acid Cycle is acetyl-CoA. Although biochemical literature very often treats oxaloacetate and its precursors—succinate, fumarate, and malate—as substrates "entering" the cycle, these compounds are not actually consumed in the tricarboxylic acid cycle. Oxaloacetate is completely regenerated, which is why it is referred to as a regenerating substrate. For the catalytic cycle to function, it is essential that the regenerating substrate is always available in the required amounts and that its concentration can be readily increased whenever the cycle reactions need to be accelerated. Under normal conditions, oxaloacetate is produced in whatever quantities are necessary for the tricarboxylic acid cycle from phosphoenolpyruvate or Pyruvate [equation (8-2)]; both of these compounds are readily available products of sugar METABOLISM.
In Bacteria and green plants, the synthesis of oxaloacetate is mediated by phosphoenolpyruvate carboxylase [equation (7-79)], an enzyme subject to extensive regulatory control. In animal Tissues, pyruvate carboxylase plays a comparable role [equation (8-2)]. The latter enzyme remains nearly inactive in the absence of the allosteric effector acetyl-CoA, which is why it went unnoticed for many years. High concentrations of acetyl-CoA lead to full activation of the enzyme, ensuring the synthesis of oxaloacetate at levels high enough to sustain the cycle. It should be noted, however, that the concentration of oxaloacetate in Cell/35.html">Mitochondria is extremely low—only 2∙10-7 to 4∙10-7 M (20—40 molecules per mitochondrion) [16].
Box 9-D
The Use of Isotopic Tracers in The Study of the Tricarboxylic Acid Cycle
The initial application of isotopic tracers to the Study of the tricarboxylic acid cycle—and indeed one of the earliest in The history of biochemistry—was carried out by Wood and Werkman at the State University of Iowa (USA)a. Their objective was to investigate the Fermentation of glycerol by propionic acid bacteria, a process with no apparent connection to the tricarboxylic acid cycle:
Class="center">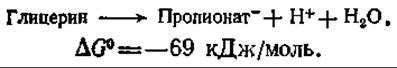
During fermentation, The formation of small quantities of succinate was observed. Based on simple balance measurements of the fermentation process, it was hypothesized that CO2 is incorporated into oxaloacetate, which is subsequently reduced to succinate. This finding was reported in 1938. As we now know, this pathway is indeed an essential step in Propionic Acid Fermentation (Section E, 3). At that time, the 14C isotope was not yet available; however, using a mass spectrometer designed by Nier, it was possible to detect the presence of the stable isotope 13C. Wood and Werkman developed a thermal diffusion Column to produce bicarbonate enriched with the 13C isotope and set up the mass spectrometer. By 1941, it was definitively established that Carbon dioxide is incorporated into succinate in bacteriab.
It was suggested that the incorporation of CO2 into succinate might also occur in animal tissues. To test this hypothesis, Wood investigated the metabolism of pigeon Liver preparations, adding malonate to block succinate dehydrogenase (Box 9-C). To the researcher's surprise, the accumulating succinate contained no 13C isotope. Soon thereafter, however, it was demonstrated that CO2 is incorporated into the carboxyl group of $\alpha$-ketoglutarate adjacent to the carbonyl group. Upon subsequent conversion into succinate, this carboxyl group is lost (Fig. 9-2), which explains the absence of 13C in the succinate. Historically, it is noteworthy that these observations were misinterpreted by the majority of biochemists of the time, who consequently agreed that citrate does not participate in the tricarboxylic acid cycle.
Because citrate is a symmetrical compound, it was assumed that upon incorporation of the 13C isotope into citrate, the label would always be distributed equally between its two terminal carboxyl groups. If so, 13C would inevitably be incorporated into succinate as well. It was not until 1948 that Ogston formulated the concept that binding a substrate at a minimum of three points enables Enzymes to attack symmetrical substrates asymmetricallyc. In other words, an enzyme can synthesize citrate in such a way that carbon atoms originating from the acetyl-CoA molecule will always end up exclusively in one of the $\text{CH}_3\text{COOH}$ groups flanking the prochiral center (Chapter 6, Section D, 2).
In recent years, the use of various isotopic tracers has helped elucidate the complete Stereochemistry of the tricarboxylic acid cycle reactions (Chapter 7, Section K, 2, g). Some of these findings are indicated in Fig. 9-2 by asterisks (*) and superscript plus signs (+).
a Wood H. G. In: The Molecular Basis of Biological Transport (J. F. Woessner, Jr. and F. Huijing, eds.), pp. 1—54, Academic Press, New York, 1972.
b Wood H. G., Werkman C. H., Hemingway A., Nier A. O., JBS, 139, 377—381 (1941).
c Ogston A. G., Nature (London), 162, 963 (1948).
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.