Protein Chemistry - Part 1 - General Protein Chemistry - Ashmarin, I. P. 1968
Determination of the size and shape of protein molecules
Viscosity of protein solutions
Although viscosity measurements of protein solutions do not directly provide information about the size and shape of macromolecules, this method is one of the simplest approaches for studying molecular parameters. Based on the viscosity measurements of solutions containing ellipsoidal and rod-shaped molecules, it is possible to calculate The ratio of the molecular length to its thickness, and for Fibrous Proteins, to determine their absolute dimensions as well. On the other hand, the viscosity of dilute protein solutions is a function of their molecular weight. Admittedly, the molecular weight cannot be determined from viscosity data alone; however, a direct correlation can be established between the molecular weight determined by other Methods and the viscosity. Finally, viscosity measurements clearly illustrate the changes in molecular Structure that occur during the Denaturation of protein molecules, their aggregation, or their dissociation into subunits.
Viscosity is a measure of resistance to shear in a fluid and can be viewed as a form of internal friction. If a moving layer of fluid imparts motion to the adjacent layer through internal friction, the force required to maintain such motion is proportional to the area of the layers and the velocity gradient between them:
Class="center">т = η ∙ g (14)
where т is the shear stress (shear stress being the tangential force per unit surface area between adjacent layers required to maintain relative motion), g is the velocity gradient or shear rate, and η is the proportionality factor known as the coefficient of viscosity of the liquid. The term viscosity is commonly used instead of "coefficient of viscosity." The unit of viscosity in the CGS system is the poise (P), or g/cm∙s.
Viscosity is determined using various viscometers, the simplest of which is the Ostwald viscometer (Fig. 34). An aqueous solution is allowed to drain from pipette 3 through capillary 4, and the time required for the meniscus to drop from point 1 to point 2 is measured. If the viscosity of the protein solution does not differ too greatly from that of Water and if the capillary diameter is properly selected, the viscosity η is directly proportional to the efflux time t and the density of the liquid d:
η = С ∙ t ∙ d, (15)
where C is a constant that depends on the dimensions of the viscometer.
A transformed form of this equation is frequently used instead:

where v is the so-called kinematic viscosity (η is termed dynamic viscosity). Thus, kinematic viscosity is proportional to the efflux time; the unit of kinematic viscosity is the stokes (St), where 1 St equals 1 cm2/s. If η0 is the viscosity of water and η is the viscosity of the protein solution, the relative viscosity is given by


Fig. 34. Ostwald viscometer (from Haurowitz, 1965). Explanations in the text.
It can be seen that the relative viscosity is independent of the constant C, which is a function of the capillary diameter. Since the viscosity of a protein solution is always greater than that of water, the relative viscosity will always exceed unity. The difference between this value and unity is called the specific viscosity and represents the fraction of viscosity associated solely with the solute molecules:

At high solution concentrations, interactions occur between the dissolved protein particles, which are particularly strong for fibrous molecules; therefore, to characterize macromolecules, viscosity measurements must be performed in highly dilute solutions. Since the viscosity of dilute solutions differs very little from that of water, the Procedure is as follows. Viscosity is measured at several concentrations, the value
ηsp/c is calculated each time, and a plot of this value versus c is constructed. Extrapolation yields the value of ηsp/c at c = 0. This extrapolated value is called the intrinsic viscosity [η] when concentration is expressed in g/100 mL, or the limiting viscosity number [η] when concentration is expressed in g/mL:
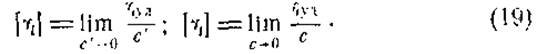
The term "intrinsic viscosity" is not entirely precise; [η] is not actually a viscosity and does not have the dimensions of this quantity, but rather is a value proportional to the volume occupied in solution by the solute molecules. To clarify this, we must examine METABOLISM/2.html">THE CONCEPT OF the "viscosity increment."
Einstein theoretically calculated that the viscosity of very dilute solutions of spherical particles is determined by the formula:

where N is the number of particles, v is the particle volume, and V is the total volume of the solution. The expression Nv/V = Φ represents the volume fraction of protein particles in the solution. Transforming the equation, we obtain:
ηsp = 2,5Ф. (21)
Somewhat later, this equation was generalized by Simha for ellipsoidal particles

where η is the viscosity increment*, which equals 2.5 for spherical particles of Globular proteins. Since the intrinsic viscosity [η] is expressed in terms of weight concentration and the viscosity increment in terms of volume concentration, these quantities are related by the equation

where  is the partial specific volume at infinite dilution, i.e., the increase in solution volume upon adding a unit weight of anhydrous protein to a sufficiently large volume of solvent. The value of
 for proteins typically ranges from 0.69 to 0.75.
The viscosity increment depends on the axial ratio of the equivalent ellipsoid of revolution. For prolate particles with an axial ratio of f = a/b > 1.5, this dependence is described by the formula
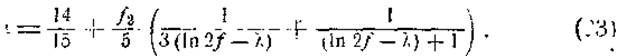
* The viscosity increment is frequently denoted by v. However, we have used a different notation to avoid confusion with the kinematic viscosity mentioned earlier.
For oblate ellipsoids, λ is 1.5, and for prolate ones, it is 1.8. Thus, knowing [η] and v, one can easily calculate the viscosity increment and the axial ratio, thereby determining the molecular shape. Furthermore, intrinsic viscosity can also be used to estimate molecular weight. Based on measurements of polymers with medium and short chain lengths, Staudinger established that
N = КМ, (24)
where K is a constant that depends on the specific Properties of the polymer and the solvent. It can be estimated approximately by measuring [η] for a protein of known molecular weight.
More precise measurements have shown that the Determination of the Molecular Weight of rod-like particles is better described by the formula
[η] = KMa, (25)
where a ranges from 0.5 to 1.5. The main difficulty in determining molecular weight from viscosity measurements is that the quantitative relationship between them holds true only for preparations that are homogeneous in molecular weight. In addition, when measuring the Viscosity of Protein solutions containing thread-like molecules, one must account for the phenomenon known as thixotropy. This consists in the fact that upon standing, a sufficiently concentrated protein solution (such as Actin) transforms into a gel-like state, which can be reverted to its initial liquid state simply by shaking.
Last update: 06/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.