GENETICS - Textbook - A.V. Sivolob - 2008
CHAPTER 8. Population Genetics
FACTORS DRIVING THE DYNAMICS OF POPULATION GENETIC STRUCTURE
Genetic Drift
Population sizes are invariably finite. When a population has a relatively small effective size $N_e$ (in the absence of Selection, mutation, and migration), The formation of the gamete pool and the Gene pool of the next generation significantly increases the probability of random deviations from the mean frequency of a given allele. This process of non-directional allele frequency changes in small populations driven by stochastic factors is known as Genetic Drift.
These random fluctuations lead to unpredictable shifts in gene frequencies across generations (Figs. 8.5, 8.6). The ultimate outcome of this process is either the elimination of an allele from the population or its fixation (reaching a frequency of 100%), with The rate of this process increasing as $N_e$ decreases.
Class="center">
Fig. 8.5. Process of random change in gene frequencies over a single generation in a population of four hermaphroditic individuals, where reproduction occurs via random gamete fusion (adapted from Kimura, 1985)
The stochastic and unpredictable nature of genetic Structure changes in a given population necessitates a probabilistic approach, which is the only way to study genetic drift effectively. The probability of allele frequency deviating from its initial value can be estimated using standard deviations (σ). The variance of allele frequency is determined by the formula
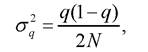
where q is the frequency of allele a in the initial ($i$-th) generation, and N is the size of the subsequent daughter ($i+1$) generation. Hence, the standard ROOT-mean-square deviation of the gene frequency in the daughter generation is
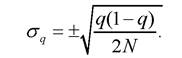
The greater the deviation of the allele frequency from its initial value, the lower its probability: the interval from q - σ to q + σ encompasses 68.27% of all possible random allele frequency deviations, the interval from q - 2σ to q + 2σ encompasses 95%, and so on.
As a result of random gene frequency changes across generations, both fixation and elimination of alleles will occur, leading to an increase in population homozygosity and a loss of Variability (Figs. 8.6, 8.7). The rate of this variability loss is given by k = 1/(2N). In other words, in a group of N individuals reproducing via random mating, heterozygosity will decrease by a factor of 2N in each generation:
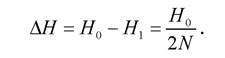
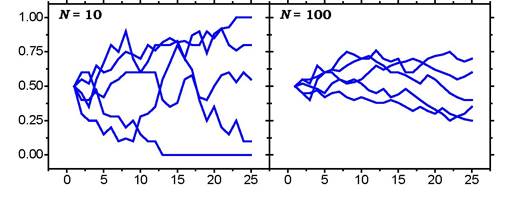
Fig. 8.6. Curves of gene frequency drift.
The abscissa represents the number of generations, and the ordinate represents the gene frequency.
The curves were obtained from computer simulations modeling populations
of 10 and 100 individuals with an initial gene frequency of 0.5
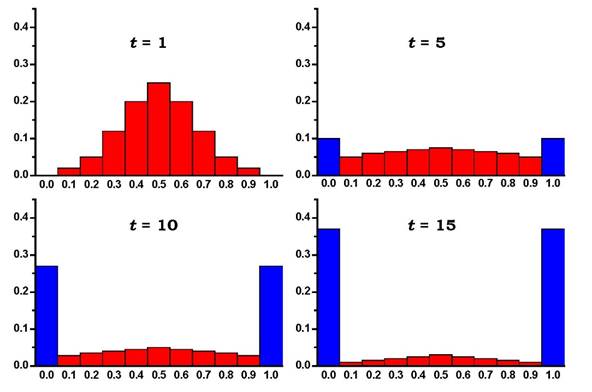
Fig. 8.7. Changes in the gene frequency distribution as a result of genetic drift: the abscissa shows the allele frequency, and the ordinate shows the proportion of populations with the corresponding frequency. Populations consist of 5 hermaphroditic individuals with random mating; the initial gene frequency (at t = 0) is 0.5. Distributions are shown for the 1st, 5th, 10th, and 15th generations. Blue bars indicate the proportion of populations in which the allele has been lost or fixed (adapted from Kimura, 1985)
Heterozygosity in a group of N individuals after t panmictic generations can be calculated using the formula
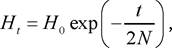
where H0 is the initial heterozygosity, and Ht is the heterozygosity after t generations.
In the same manner (i.e., at a rate of 1/(2N) per generation), genetic drift affects another measure of variability: the number of loci at which neither fixation nor elimination of an allele has occurred.
The main consequences of genetic drift are:
✵ unpredictable changes in allele frequencies;
✵ an increase in the proportion of homozygotes;
✵ gene pool depletion (loss of alleles).
Drift significantly impacts the genetic structure of a population during fluctuations in numbers, when the population size drops sharply (the bottleneck effect), and the gene pool of subsequent generations is determined by a small group of founding individuals (the founder effect). Although the population size may later increase substantially, The genes of all individuals trace back to a small number of genes that happened to be present in the founders. In particular, this applies to human populations at certain stages of Homo sapiens evolution (Chapter 7). The founder effect occurs both when a population passes through a bottleneck and when a species colonizes new, isolated areas (such as islands).
Last update: 07/08/2026
Editorial and Educational Adaptation: This material has been compiled based on the primary/original source text. The project team performed an editorial review, corrected technical inaccuracies, structured sections, and adapted the content for an educational format.
What was processed:
- elimination of formatting defects (OCR errors, structural breaks, corrupted characters);
- editorial organization of content;
- standardization of terminology in accordance with academic sources;
- verification of factual statements against the original source text.
All mentions of the author, publication year, and origin of the primary text have been preserved in accordance with the source.